Elements of Darwinism Life on Earth has evolved over billions of years by sheer chance, filtered by natural selection. So says Darwinism, the most influential idea of our time. If a rare random mutation helps DNA[1]...
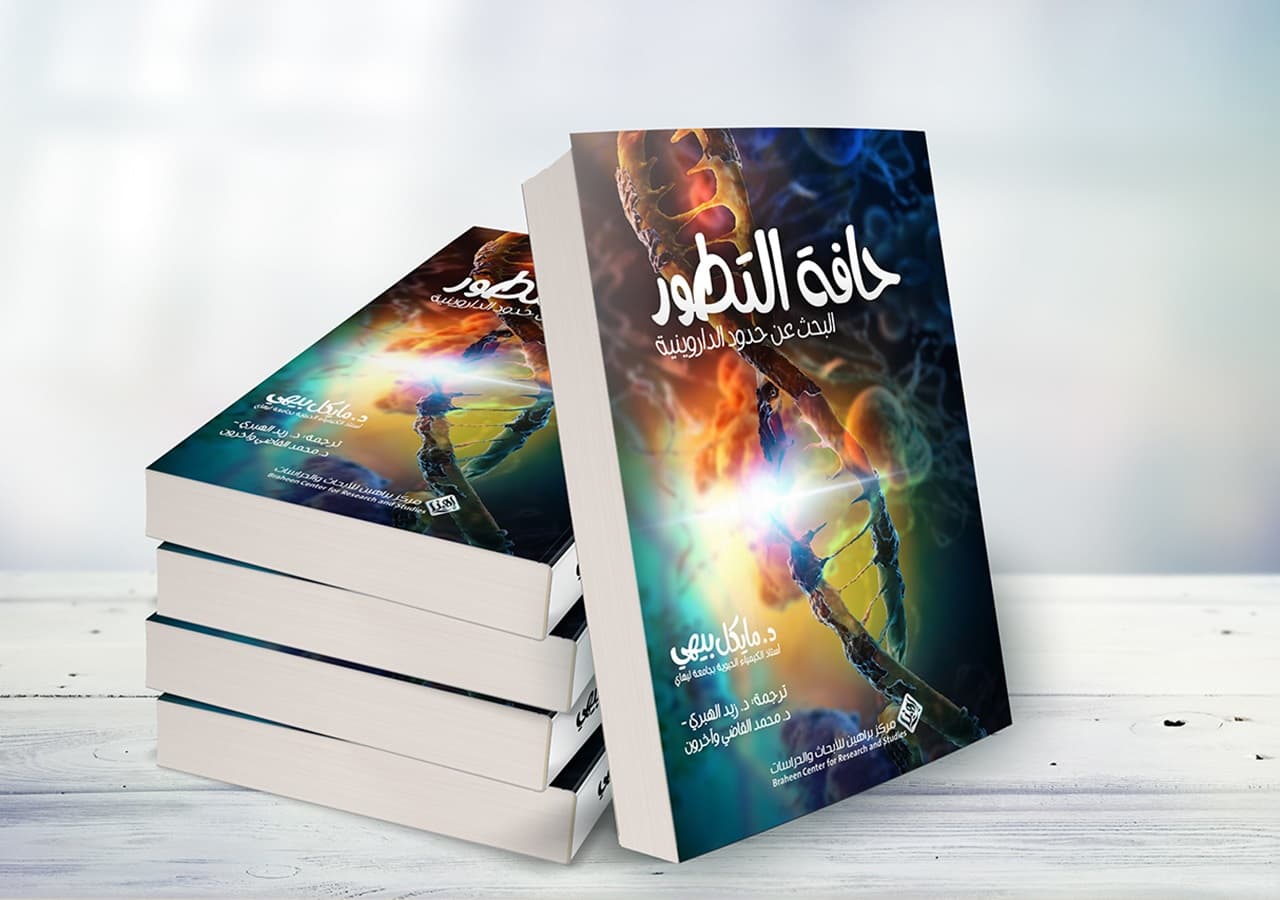
Edge of Evolution: The Search for Darwinism's Frontiers - Author's Introduction
Elements of Darwinism
Life on Earth has evolved over billions of years by sheer chance, and has been filtered out by natural selection. So says Darwinism, the most influential thought of our time. If, in the distant past, a rare random mutation in DNA[1] helped the lucky mutant to leave a larger offspring than the rest of its species, then as generations pass the species as a whole will have changed.
This is at least the claim. But is it true? To answer this question, you must examine Darwin’s theory carefully, because it is not a single concept; in fact, it is a mixture of unrelated, even quite separate, ideas. The three important ideas to consider from the outset are: random mutations, natural selection, and common descent.
Common descent is what most people think of when they hear the word "evolution." It is the saying that different types of present-day creatures can be traced back to a common ancestor. For example, two mutants and giraffes two mammalian species are both viewed as descendents of a single species from the ancient past.
This is certainly fascinating, and so it is understandable that most people view the idea of shared regression with such amazement, that they do not investigate it further. But very deeply, the interpretation of shared regression is also trivial. But alone, it doesn't try to explain how traits or ancestors themselves came to be here in the first place, or why descendants diverged afterwards. For example, rabbits and bears have hair, so the idea of co-regression just says that their ancestor had hair too. Plants and animals have complex cells with nuclei, and so they must have inherited that property from a common ancestor. But the question of how or why remains pending.
In contrast, Darwin’s proposed mechanism of evolution – the compound concept of random mutations associated with natural selection – certainly aspires for more. Linking the concepts of random mutations and natural selection is to try to explain the differences between creatures.
Let's deconstruct the compound concept. First, let's address natural selection.
The idea of natural selection alone, it just says that the most viable organisms in one species will produce offspring that are more viable than the least viable organisms. So, if the total number of species remains the same, the lineage of the most viable organisms will replace the lineage of the least viable organisms. It is no surprise that creatures that are somehow more viable (stronger, faster, or stiffer) will generally perform better in nature than those that are less viable.
The role of random mutations is the most critical aspect of Darwin's multifaceted theory. Almost all new and important in Darwinian thought is centered in the third concept. In Darwinian thinking, the only way a plant or animal can become more viable than its relatives is by preserving the occipital mutations.
Random mutations, natural selection, and common descent; three separate ideas were combined into a single theory. Because of the fusion of concepts, the question of whether Darwinism is true has several possible answers. One possibility, of course, is that those separate ideas – common descent, natural selection, and random mutations – can all be completely true, and sufficient to explain evolution. Or, they can all be true, in the sense that random mutations and natural selection are also important. Many prominent biologists of the late 19th and early 20th centuries saw shared regression as a good idea, while natural selection with random mutations as a wrong idea.
The results of recent experiments on DNA sequences – undreamed of by 19th-century scientists such as Charles Darwin – show that some distantly related organisms share apparent arbitrary characteristics of their genes[2] for which we seem to have no explanation other than that they were inherited from a distant common ancestor.[3] Secondly, there is also ample evidence that random mutations associated with life can be modified.
As we will see throughout this book, genetic accidents cause part of evolutionary change, but only part of it. As previous generations of scientists, unlike the outer envelope of life, have agreed, evidence of a pivotal role for random mutations is very bad.
In recent years, Darwinian thinkers have pushed their ideas aggressively into the arenas of public debate as a kind of reasoned theory of everything in biology; they claim that applying Darwinian principles to medicine will tell us why we get sick, and Darwinian psychology explains why some men rape and some women kill their newborns. The appeal of seeing the world through Darwinian lenses has been to humanities, law, and politics.
Either you accept the whole theory or you decide that evolution is just hype and throw it all away. Both are wrong. When we deal with a nature that is often dangerous, we cannot afford to elevate anyone’s beliefs above evidence.
The importance of finding the path
On the surface, Darwin's theory of evolution is seductively simple, and unlike many theories in physics and chemistry, it can be summarized briefly and without mathematical formulas: in each species, there are changes. For example, one animal can be bigger than its brothers and sisters, another can be faster, and another can be their brightest color. But unfortunately, not all animals born will survive in order to reproduce, because there is not enough food for all species, and there are also predators. Over time, the descendants of this organism with this lucky original mutation will be the majority in the group, and then the species as a whole will change from what it was. If this scenario is repeated again and again, the species will change completely into something completely different.
At first glance, this seems to be easy and smooth. Change, selection, inheritance (in other words, random mutations, natural selection, common descent) seem to be all that is needed. In fact, when the evolutionary story is worded briefly as in the previous paragraph, Darwinian evolution often appears as if it were a logical necessity.
On the ground, random mutations, natural selection, and shared regression can all be perfectly valid, but the Darwinian process may still be an inadequate explanation of life. For the many complex structures of life to form, the Darwinian process will have to take many consistent steps, a series of beneficial mutations that help each other successfully construct, and then perform.
The path question is as central to evolution as it is to our daily lives. In everyday life, if you walk blindfolded from point A to point B, then the problem will always vary depending on where point A is, where point B is, and what's in between. Suppose you had to walk blindfolded (and to make the example closer to the Darwinian spirit, blindfolded and drunken) from point A to point B to get a point B. Small. On the other hand, if you have to walk blindfolded from one side of a city you don't know to the top of a skyscraper on the other - across busy streets, passing hazards through entrances - you'll have innumerable problems. You'll probably stagger off the top of an entrance stairway, get on top of cars, and so on. You'll stumble into any one of thousands of local spots. Of billions of people blindfolded by strays who might be trying to do something like this.
In everyday life, the greater the distance between points A and B, and the more rugged the ground, the less likely it is to walk blindfolded, even when you follow a stupid rule like "always jump up, never back down." The same goes for evolution. In Darwin’s day, scientists were ignorant of many details of life, so it was reasonable to aspire to find evolutionary paths that would prove short and easy. But now that we know more, huge advances in modern science have shown that life is enormously complex and elegant, especially at the molecular level. The problem with Darwinism, then, is that, as with a long walk outside with blind eyes, random mutations and natural selection in a rugged evolutionary land may keep the species in genetically blocked ways, stuck at the top of small anatomical mounds, or wandering aimlessly in physiological plains, and it will never come close to winning the biological Gold Cup. If this is the case, then the mechanism of random mutations associated with natural selection will not be effective. In fact, the urgent need to jump into any evolutionary mound will constantly prevent all drunks from finding the distant top of a biological mountain.
That point is crucial: if there is no evolutionary path that is smooth, incremental, and easy to find that leads to a biological system in a reasonable timescale, the Darwinian mechanism will not work.
A peek back.
As a practical step, how far must be between biological points (a) and (b), and how rough is the path between them, before the Darwinian mechanism becomes inefficient? How can we determine when we can get to that point? Where in biology is the reasonable place to draw the line that determines the edge of evolution?
This book answers those questions, which arose because of the research I started more than 10 years ago in Darwin's Black Box. My argument was that complex, irreducibly complex structures, like some enormously complex cellular machines, could not have evolved by random mutations and natural selection.
In particular, many of the chapters in the scientific community have been set on fire by my later conclusion that these three rules are cleverly designed. Many people strongly oppose this conclusion for a variety of reasons. In this book, although my results are ultimately the same, I will no doubt find opposition from some, but I have spent most of the book's chapters drawing clues to the argument based on molecular evidence, genetic research, and – most importantly – critical studies in the field of single-cellar evolutionary changes. However, as we seek to find the dividing line of the edge of randomness, there is no need to refer to the design.
Opening the impasse.
In Darwin's Black Box I was only interested in showing that some of the elegant structures in life are beyond the range of stochastic patterns and natural selection. This book aspires to do even more. The focus here is to draw reasonable general guidelines for determining the edge of evolution; that is, to decide with some precision where Darwinian interpretations are unlikely to be accepted, not just for certain structures, but for the general characteristics of life.
Is the pile of stones next to the outer wall a table, or a religious structure to accept sacrifices? Is the land next to the wall a remnant of the field ploughing? Where are the city’s borders? Where are the traces of civilization and where does raw nature begin? A decision on these marginal issues will be a much more difficult task, and the results will inevitably be more tentative.
Although they have to worry about the impact of physical processes on the artifacts they study, they usually don’t concern themselves too much with biological effects. But in our search for where Darwinian extremes lie, unique biological processes do, of course, come to the scene. Random mutations in DNA can be likened to random occurrences of inanimate events.
Life has existed on Earth for billions of years. During this time, huge numbers of organisms have lived and died. Darwinists hypothesize that the ferocious conflicts between different breeds throughout the ages led to biological “arms races”; competitive improvements to biological warfare capability are similar to the advanced 20th-century arms race between humans in the United States and the Soviet Union.
Modern laboratory studies of random mutations and natural selection have suffered from the inability to examine large numbers of creatures. Usually, even with heroic efforts by the best investigators, it is relatively few organisms that can be studied only, and for a relatively short period of time as well, after which the changes in a few selected traits are pursued. At the end of such studies, while some interesting results are available, it is usually impossible to generalize.
Thus, in the absence of crucial laboratory tests, most biologists operate spontaneously within the Darwinian framework, simply assuming the validity of the unprovable. Unfortunately, this leads us to the habit – understandable, but nevertheless destructive – of forgetting the difference between what has been postulated and what has been proven.
Getting out of the theoretical predicament will require precise evolutionary data at the genetic level from a huge number of organisms that are under constant pressure of natural selection. That data simply wasn't available in the past. But it's available now.
Jumps and Borders
Even just ten years ago, any attempt to determine the edge of evolution with any form of precision was almost impossible. Only a little was known. But with the powerful advance of science, especially in the last decade, the task became possible.
The greatest difficulty in evaluating an evolutionary theory like Darwinism can be summarised as follows; while we can easily detect significant changes in plants and animals, the reasons for these changes remain unclear. Darwin and early scientists, for example, could have examined changes in beaks of birds, but could not figure out what caused these modifications. As we get closer to our days, mid-20th-century scientists have found that some bacteria have developed antibiotic resistance, but they don’t know what exactly gave them that ability. Only in the last half century has science shown that these apparent changes are caused by mutations in hidden molecules, proteins and DNA. The only way to get a realistic understanding of what random mutations and natural selection can actually do, is to track changes at the molecular level. The right evaluation of Darwin’s theory certainly requires an assessment of random mutations and natural selection at the molecular level, and caring about that is pivotal.
The good news is that with a lot of foresight and effort, modern science has developed the tools to do this. The triumph of the 20th-century DNA strip is to demonstrate one of the requirements of Darwin's theory; the fundamental basis of differences. We now know that differences in organisms depend on subtle changes in DNA structure (for a summary of DNA structure see Appendix A). What's more, scientists have catalogued innumerable ways in which DNA changes occur. Other times virus-like active DNA elements can insert copies of themselves elsewhere in the genome, and sometimes pull other parts of the DNA with them. Natural opportunities to manipulate the organism's DNA are practically unlimited.
The hard work of many scientists has shown us not only the fundamental basis of variation, but also the rate of mutations in which fairly satisfactory results have been achieved. As a rule, DNA transcription occurs most correctly. On average, the error occurs only once in every hundred million (almost) nucleotides copied in a generation. But there are exceptions. In viruses such as HIV, the rate of mutations accelerates dramatically.
Another pivotal advance in our ability to properly test Darwinism came from our knowledge of DNA sequences. In the last few decades, the amount of DNA sequences that have been known has steadily increased, and the number of organisms in which DNA sequences have been known has swelled.
But all this scientific progress is still not enough to draw firm conclusions about Darwinian evolution if we do not study enough organisms. The larger the number of organisms, the greater the chance of random mutations finding beneficial change and passing it on to natural selection, the tougher the conclusions about what Darwinism can do. Studies of animals like sparrows, at most, can trace the lives of hundreds of them.
The natural world is teeming with organisms, of course. There could be billions of mammalian species on the planet at some point, like humans and mice. In the seas there are huge numbers of fish. While labs can't grow enough organisms to do a reasonable treatment of Darwinian evolutionary abilities, nature doesn't have those problems.
Evolution from a common ancestor, through changes in DNA, is very supported by evidence. It may be random, or it may not be. Scientists who trace DNA sequences in humans and identify beneficial mutations – as opposed to our natural enemies, for example – do not study DNA in one person, thanks to evolution. They actually observe the results of a conflict that has lasted for more than a thousand years and involved millions of human descendants.
The Definitive Evidence in Darwinism
The single best test of Darwin's theory is the history of malaria; thanks to its sheer numbers, its random reproduction rates, and our knowledge of genetics, malaria has emerged. The bulk of this book will focus on the disease. Many parasitic diseases infect humans, but historically malaria has been the greatest affliction, and one of the most thoroughly studied. For ten thousand years parasitic mosquitoes have caused disease and death in vast areas of the earth. These mutations have been popularized by Darwinists as one of the best and clearest examples of Darwinian evolutionary abilities.
But, as we shall see, since the cover has revealed the molecular changes that cause malaria resistance, it turns out that it tells a very different story than Darwinists expect; one that emphasizes the dissonant confusion involved in blind research. Malaria offers one of the most important examples of Darwinian evolution, but points in two separate directions; what Darwinism can and cannot do.
Because it has been widely studied, and because of the astronomical numbers of organisms included in that study, the evolutionary conflict between humans and our archaic opponent (malaria) is the best and most reliable basis for forming perceptions of the ability of random mutations and natural selection. Few other sources of information come close, and as we will see, this small number also tells similar stories.
Important explanation for the reader: Unfortunately, in order to fully understand and appreciate the difficulties of random mutations, and how the battle of humans with malaria illustrates them, we must prejudice ourselves and immerse ourselves in the details of the battle at the molecular level. I will make every effort to minimize technical details as much as possible, some of which will be confined to appendages. But there is no way to escape the fact that this topic requires technical details.
Although the number of malaria cells is huge, it is much lower than the number of organisms found on Earth. However, as I will explain, the explicit extrapolation from malaria data allows us to establish reasonable experimental limits on what we can expect from random mutations, even for all life on Earth in the last billions of years. Not only that, but studies of the E. coli bacterium and the HIV virus (the virus that causes AIDS) provide clear confirmation of the lessons learned. Viruses contain far less genetic material, but they mutate very quickly, and there are so many copies of them, that HIV alone – in the last 50 years alone – has undergone more than all the cells have been exposed to since the beginning of the world from at least some types of mutation.
Most of this book will focus on cellular and molecular processes, but in the other two chapters I will go further. In recent years, while science has made a remarkable leap, it has discovered some basic molecular details in the growth of different animal species, and has therefore drawn some conclusions about the limits of using random mutations in interpreting animal life traits.
Flashes off the edge.
One of the difficulties of writing a book to check the efficiency of Darwin's theory is that some people mistakenly conclude that you reject it altogether. It's time to clarify, to go beyond such preconceptions. Random mutations are a perfectly adequate explanation for some of life's characteristics, but not all of them. This book looks for the line between random and non-random that defines the edge of evolution. Think of these examples:
In the middle of the 20th century, a miracle occurred, and drugs were discovered that could cure this majestic disease, and hopes for its complete eradication were raised. But within ten years, malaria developed drug resistance. New drugs were developed and put into battle, but the results were not proven much.
* On the other hand, there is sickle cell disease. Although it is considered a complete disaster in the United States, there is a bright side in Africa. The transmission of the disease requires two copies (one from the father and one from the mother) of the mutated sickle cell gene. People with one copy do not get sick, but are resistant to malaria, and thus survive the same time when others die. The gene that carries the sickle cell mutation originated in Africa about ten thousand years ago.
On the one hand, there is HIV. The price that humans have paid for AIDS in the current era is similar to what happened in the Middle Ages with the Black Death. Recent research has developed a number of drugs to fight AIDS, but after a short time - months, sometimes days - they have always lost their effect. The reason is Darwinian evolution. The HIV genome, the virus that causes AIDS, is a tiny snippet of RNA, barely equals a millionth of the size of a minute. Here, evolution defeats medicine.
On the other hand, there is Escherichia coli, which naturally resides in the human intestinal tract. Escherichia coli has also been the bacterium of choice for study in the lab for more than a century. Its genetic and biochemical aspects are more understandable than any other organism. During the last decade, Escherichia coli has been the subject of the most extensive laboratory evolutionary studies ever conducted. By multiplying seven times a day, the bacterium has been growing steadily in vials for more than 30,000 generations. 30,000 generations are worth roughly a million years in human life. Although some peripheral details of some systems have changed over the past 30,000 generations, the bacterium has repeatedly dumped pieces of its genetic heritage, including its ability to form some of the most basic components of RNA. In contrast, nothing close to that discarded elegance has been built. The lesson of Escherichia coli is that it is easier to tear things down than to develop.
On the one hand, there is the Antarctic Notothiniwadai, which survives in temperatures supposedly freezing its blood. Studies have shown that there have been cumulatively small genetic changes in the fish’s DNA over the past 10 million years, giving it the ability to create a strange new type of antifreeze; an antifreeze that sticks to the ice core and prevents it from growing.
On the other hand, there is malaria (again). Fierce parasitic malaria – the same evolutionary dynamo that human drugs don’t affect – has a deadly vulnerability; it will only grow in its family mosquito at very high temperatures, and is therefore mainly confined to the tropics.
Somewhere in the middle of examples like this, the edge of evolution lies.
[1] DNA is short for Deoxyribonucleic acid, which is a large molecule found within the cells of all living organisms and many viruses and contains genetic information that allows the work, reproduction and growth of these organisms, and in short we will replace it with DNA or DNA in the rest of the book.
[2] The author refers here to pseudogenes, parts of the genetic material that are thought to be dysfunctional because they lose their ability to code for a protein or because they are no longer expressed in the cell.
[3] Behe will expand on his vision of a common ancestor in Chapter 3, commenting on the issue in the publisher's introduction, and will also comment on it in its placement.
A genome (single genome) or genetic content or sum is the complete sequence of DNA (or RNA in the case of RNA viruses) of an organism.
Nucleotide is a basic unit of DNA and RNA; it serves as the basic letters by which genes are written that transmit the child's descriptions from mother and father.
- Dr. Michael Behe.
—
Source: Brahin Center website - Posted on 2019-01-19 (archived at the Internet Archive)
https://braheen.com/publications/intros/حافة-التطور-البحث-عن-حدود-الداروينية-مقدمة-المؤلف